top of page


The canopy of a pūriri tree.
Mature pūriri tree on the Thames Coast. Photo by Gabriela V.

A quintessential image of rural New Zealand - a gnarly, solitary, old tree in the middle of a paddock, refusing to succumb to less-than-favourable circumstances; a form of botanical tenacity, one could say.


The species in question is the beautiful, invincible pūriri (Vitex lucens) - a sacred, spiritual tree, a symbol of joy for the Māori people of Aotearoa, New Zealand.

This mighty, endemic, evergreen tree is a keystone species, selflessly supporting countless other organisms that live both on and off it. The pūriri tree is among the longest-living tree species here in Aotearoa. Taketakerau - a sacred pūriri near Ōpōtiki - is estimated to be between 2,000 and 2,500 years old.


Vitex lucens is the only member of the Vitex genus in New Zealand and belongs to the mint family (Lamiaceae), which also includes many herbs such as basil, thyme, oregano, mint, lavender and sage but also tropical hardwood trees such as teak.

Most often found in coastal and lowland forests in the northern North Island as far south as Taranaki, generally on fertile or volcanic soil. Pūriri trees can grow up to around 20m in height and around 1.5m in diameter. Their light-coloured smooth bark is juxtaposed by dark green, shiny, palmately compound leaves that most often have 5 leaflets. If you look very closely on the underside of the leaves , you will be able to spot domatia which are located between the secondary veins and the midrib. These are tiny chambers produced by the plant that may be occupied by arthropods in what can be a mutualistic relationship.


The underside of a pūriri leaf showing domatia.
Domatia on the underside of a pūriri leaf. Photo by L Jensen. https://www.nzplants.auckland.ac.nz/en/about/seed-plants-flowering/lamiaceae/vitex-lucens.html

The pūriri tree is one of a few species that are either in flower and/or have fruit present throughout the year and as such is an invaluable food source for other species. The bird pollinated flowers are an attractive pinkish red colour, curved and tubullar in the lower part then spread into asymmetrically arranged petals.


The fruit (drupes) are more or less spherical, bright red, and are a favourite food of the New Zealand wood pigeon, the kererū. So fond are these birds of this juicy delicacy, that there has been anecdotal evidence of them getting intoxicated after gorging on the fruit and falling of the trees as a consequense. This tipsy behaviour is the result of the alcohol-producing fermentation that takes place in the bird's crop when, after their feast, they sit on a branch in the sun for long periods of time.


Kererū New Zealand wood pigeon. Photo by Jonas Patrman.
Kererū, New Zealand wood pigeon. Photo by Jonas Patrman.

Pūriri tree with its fruit.
The fruit of the pūriri tree, so irresistible for the kererū. Photo sourced from: https://en.wikipedia.org/wiki/Vitex_lucens

The pūriri tree is a sacred tree for many tribes; it was used as a burial site for chiefs or a person of high mana.

Its leaves and bark were traditionally used in Māori medicine (rongōa) to treat skin infections, sprains, and sore throats. The yellow flavonoid dye was used to stain harakeke (flax) fibres for weaving. Its heavy and dense wood was used to make garden tools and weapons.


One of the species that is associated with pūriri trees is the pūriri moth (Aenetus virescens), also called ghost moth or pepetuna. It is New Zealand's largest moth, with a wingspan of up to 150mm.


Pūriri moth
New Zealand's largest moth, the pūriri moth. Photo by © strewick https://www.inaturalist.org/taxa/409639-Aenetus-virescensZealand's

The tiny larva first feeds on fungi growing on rotting logs, then climbs a live tree, burrows into the trunk, and eats away a diamond-shaped area of bark and sapwood around the opening. After around seven years of feeding on the nutritious callus tissue, it undergoes a metamorphosis and turns into a moth. The bright green adults then fly off to find a mate. At this stage, it was regarded by Māori as a type of ghost and thought to serve as a spiritual messenger. The adult moth lacks a mouth and digestive system and so survives solely on the energy reserves it stored during its caterpillar phase. Its sole purpose now is to reproduce, and lay thousands of eggs, all this within two days, after which it perishes.


Source:

Nature guide to New Zealand forest (Dawson, J. & Lucas, R. 2000, Random House New Zealand)

The Meaning of Trees (Vennell, R. 2019, HarperCollinsPublishers New Zealand)

New Zealand Plant Conservation Network 2025. Retrieved from http://www.nzpcn.org.nz

iNaturalist NZ. Retrieved from http://www.inaturalist.nz

University of Auckland. Retrieved from http://www.nzplants.auckland.ac.nz

A garden ornament adorned with lichens.
Lichen-adorned garden ornament at Mahara Sculpture Park and Pottery. Photo by Gabriela V.

In New Zealand, we are extremely fortunate to host around 10% of the world's population of lichen species. Close to 2,000 described species with more waiting to be discovered.

These plant-like lifeforms are in fact an astonishing example of how two (or more) completely different organisms can symbiotically work together for mutual benefit. The fact that lichens can be found in almost any habitat anywhere on the planet is a testament to their success story.


Lichens are a composite organism of algae or cyanobacteria (photobionts) and fungi (mycobiont). Scientists also believe that in majority of lichens, a third partner enters this symbiosis, an order of basidiomycete yeast. It is thought that these yeast cells play an important role in the formation and the shape variation of the cortex of the thallus (the body, vegetative tissue).


A schematic cross section of foliose lichen.
Schematic cross section of foliose lichen: (a) The cortex is the outer layer of tightly woven fungus filaments (hyphae) ; (b) This photobiont layer has photosynthesising green algae; (c) Loosely packed hyphae in the medulla; (d) A tightly woven lower cortex; (e) Anchoring hyphae called rhizomes where the fungus attaches to the substrate http://en.wikipedia.org/wiki/Lichen#/media/File:Lichen_cross_section_–_heteromeric_thallus.svg


The algae or cyanobacteria (photobionts) live among the filaments (hyphae) of the fungi.

The fungi benefits from the carbohydrates produced via photosynthesis by the photobionts, where the algae may provide up to 80% of their sugar production to the fungus.

In return, the filaments of the fungi provide protection from the environment, absorb water and minerals, and provide anchorage and extended surface area for photosynthesis.

They reproduce sexually , like other fungi, producing spores which then need to meet with a compatible algal partner to form a lichen, or asexually where a piece of lichen would break off, new lichen can grow from that fragment.


A miniature ecosystem of lichens growing on a timber fence.
An astonishing variety of shapes, colours, and sizes, lichens create their own miniature ecosystems. Photo by Gabriela V.

Lichens are pioneer, keystone species, often among the first ones to settle in places lacking soil. They play an important yet often overlooked role in all ecosystems. These living organisms are not parasites; instead, they absorb all the nutrients and sunlight straight from the atmosphere, using their host only as a substrate surface for anchorage. Many lichens are sensitive to environmental disturbances and can be used to asses air pollution.


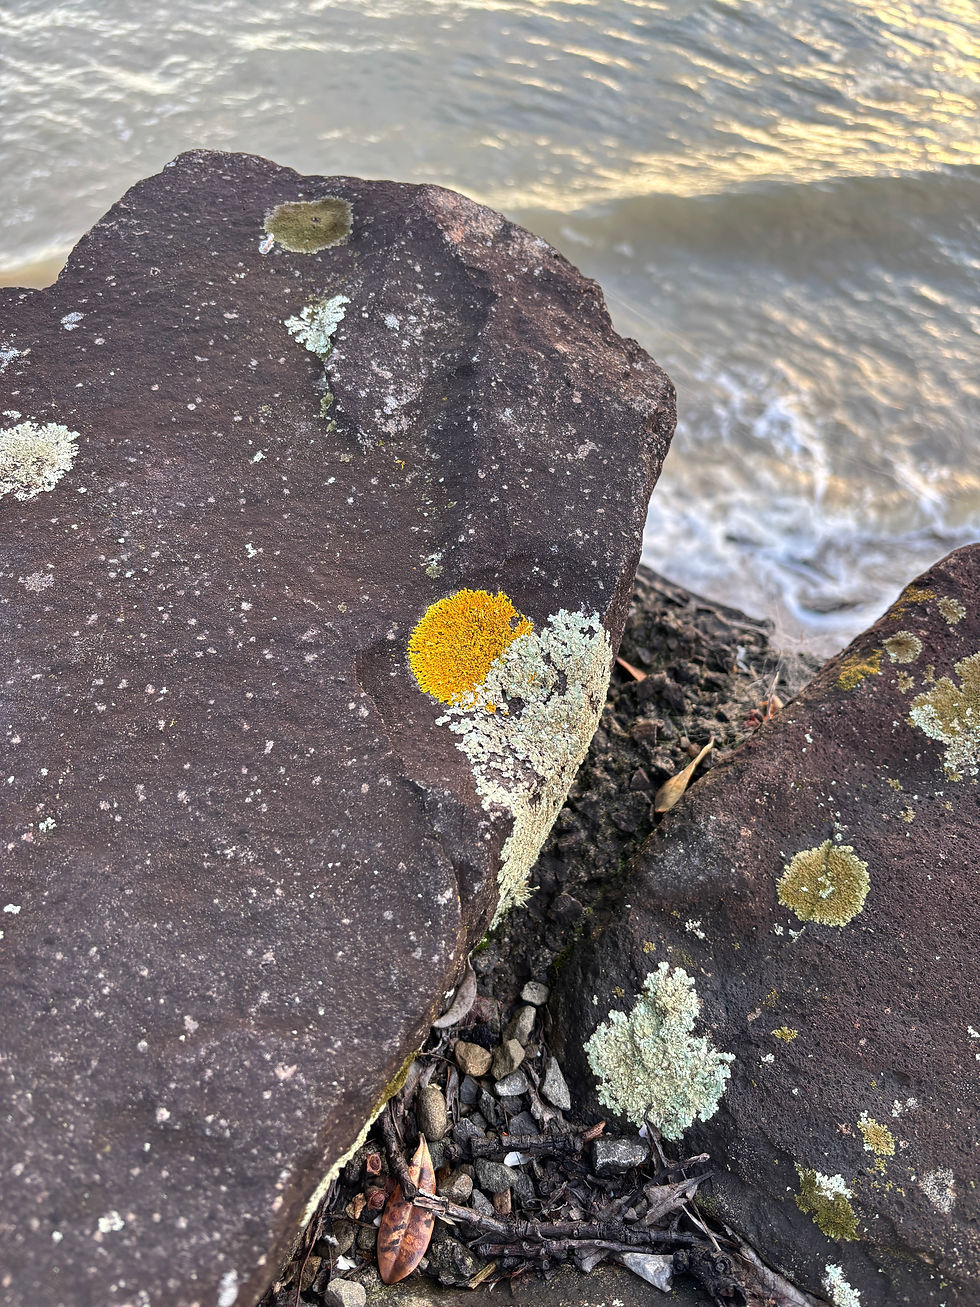
Crustose species of lichen growing on a rock in the harsh coastal environment.
Selection of crustose lichens thriving in the harsh coastal environment. Photo by Gabriela V.
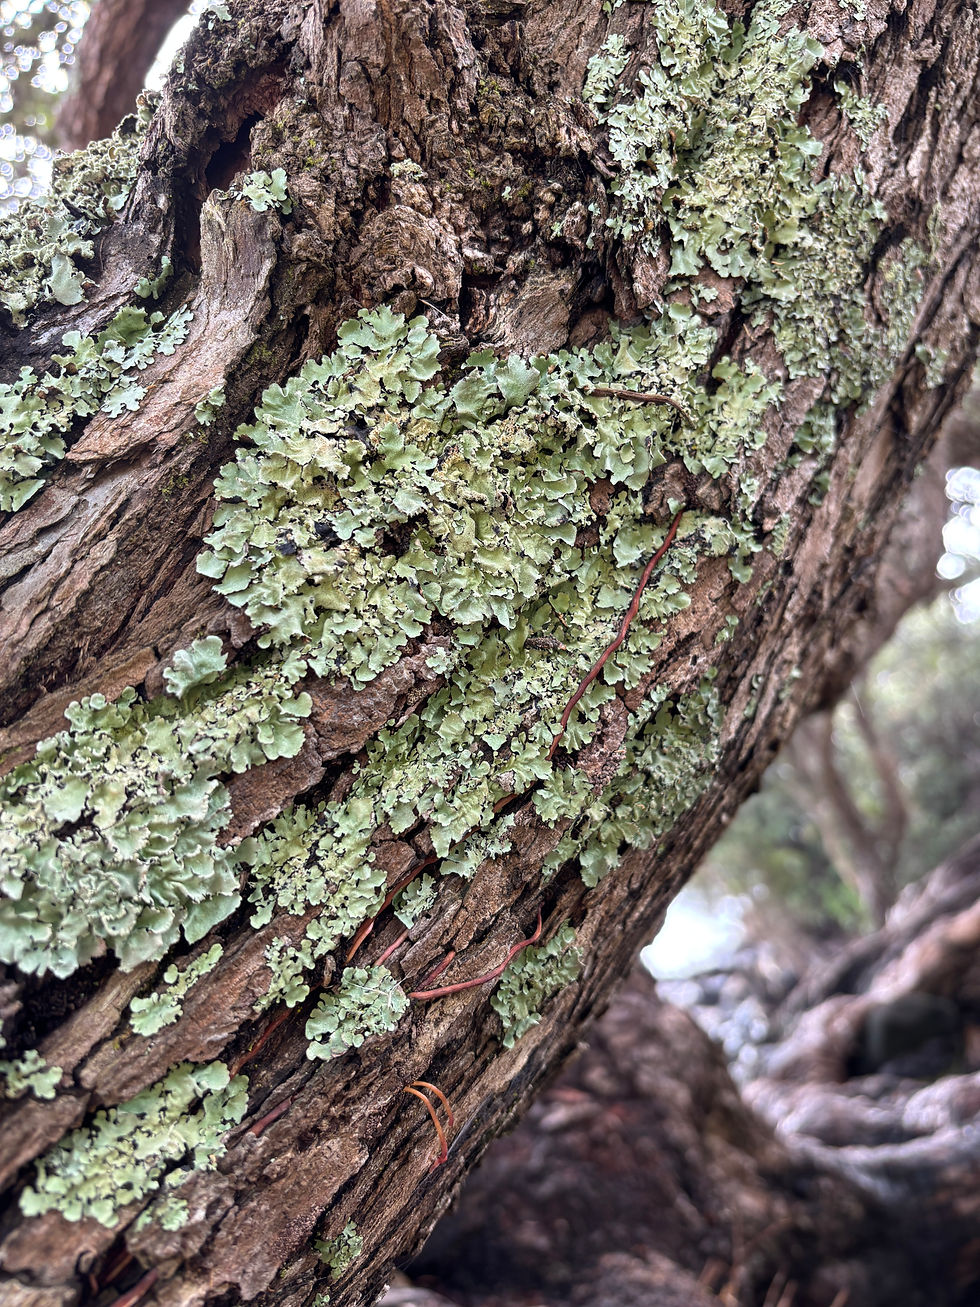
A foliose species of lichen on a pōhutukawa tree on the coast of the Coromandel Peninsula.
A pōhutukawa tree on the coast of the Coromandel Peninsula, decorated with a foliose lichen species. Photo by Gabriela V.

The ability to survive periods of extreme desiccation by going into a state of metabolic suspension (cryptobiosis) makes them extremely resilient. Lichens have even survived exposure to outer space!

They are able to manufacture protective chemicals; over 1000 are known, some of them potentially useful to humans. Though lichens are consumed by many different cultures across the world, it is important to know that certain lichens are poisonous and many contain mildly toxic secondary compounds.


Some animals, such as reindeer living in the Arctic Circle, may eat lichens; while the larvae of many Lepidoptera species feed only on lichens. It is also utilised as a nesting material by northern flying squirrels.

The northern flying squirrel in flight.
The northern flying squirrel Glaucomis sabrinus is strictly nocturnal and uses lichens as nesting material. https://extension.psu.edu/protected-species-in-pennsylvania-northern-flying-squirrel

Historically, humans have utilised lichen pigments to create dyes, with reports dating back nearly 2,000 years. The well-known pH indicator test (litmus) uses a dye extracted from the lichen Roceella tinctoria. .


With their very slow growth rate of less than a millimetre per year, they are considered to be among the oldest living organisms. One specimen of Rhizocarpon geographicum on East Baffin Island has an estimated age of 9,500 years.

Lichenometry, a geochronological dating technique where a crustose species of evenly slow-growing lichens like Rhizocarpon geographicum are used to estimate the age of exposure of rock surfaces is sometimes used for dating events in the past 1,000 to 10,000 years.


It's fair to say that there is still a lot to be discovered about lichens, and that fact is very exciting!

Languorously perched among trunks and branches, a community of plants threads through the forest canopy, both emerging from and generating ecological niches in an ethereal aerial ecosystem.


As epiphytes, these heavenly bodies grow comensally, benefitting from an association with a phorophyte, supporting plant host, without harming it. Distributed vertically, they access light and derive moisture and nutrients from the atmosphere and canopy soils through specialised morphological adaptations. The humus-rich arboreal soils in which these draped and canting flora grow is composed entirely of the decomposed leaf litter and exfoliated bark of the trees on which they perch, and of the epiphytes themselves. Native host trees can similarly develop adventitious roots in response to these pocketed soils, accessing more nutrients and developing greater resilience, particularly during periods of drought, than terrestrial species.


In New Zealand, 58 vascular plant species, those with conductive xylem and phloem tissue, are considered typical or habitual epiphytes, observing an entire life cycle above ground. As such, they dominate epiphytic plant associations. These include orchids, ferns, herbs, and shrubs.


Occasional species (19) ordinarily grow terrestrially but may occasionally grow as epiphytes in trees or tree ferns and, once established, can grow to maturity. Conversely, ephemeral epiphytes (20) are often seedlings of trees or shrubs that establish as epiphytes but die before reaching maturity, as limited by resource availability or access. Hemi-epiphytes (11), taproot epiphytes, are trees that establish on other trees, tree ferns, or shrubs and then grow a taproot toward earthly soils, eventually enabling the species to grow independent of its original host, often evidenced by an irregular form- e.g. northern rātā (Metrosideros robusta).


Observed in both humid upland regions and exposed marginal forest, the geographical distribution of a species is associated with climate; distribution within the forest and forest type; exposure to wind and solar radiation; and the bark properties determining surface adherence. Densely shaded podocarp forests contain the greatest diversity of epiphytes, their reduced light and high-moisture conditions the most conducive for these vulnerable and dependent plants. Damp and protective rimu-dominant forests contain most, if not all, typical epiphytes. Largely generalists, there are no exclusive plant associations among the treetops, but the strongly horizontal branch systems of rimu (Dacrydium cupressinum) and hīnau (Elaeocarpus dentatus) accommodate the most epiphytes of all native trees. The more open and circulating canopies of beech, pōhutukawa, or rātā-tawa forests exhibit the least diversity, referring to the environmental conditions that limit epiphytic growth. Stands of Leptospermum have similarly low populations, although species diversity improves as more small trees and tree ferns arise, often aligned with increasing piripiri, filmy fern (Hymenophyllum sanguinolentum), and taupeka, comb fern (Notogrammitis heterophylla).


Epiphytic plant succession, the gradual and directional process in which community dynamics develop over time, originates with pioneering non-vascular lichens, bryophytes (mosses), and liverworts, which absorb water directly through simple leaves or cortices (moss and lichen, respectively). As these layer and accumulate moisture and organic matter, they facilitate a dampening microenvironment wherein more drought tolerant filmy ferns and orchids arise. Once established, further population and species diversity increase.


As desiccation greatly disadvantages epiphytes, adaptations to collect and conserve water are fundamental to their habit. Morphologies therefore include epiphytes with either no special means of protection against evaporation, protected epigeal parts (stems, leaves), or specialized adaptations for absorbing and retaining water. Reduced roots systems and limited soil resources influence the channeling forms of nest epiphytes which retain water and humus at the base of the plant, encouraging rootlets to ramify into the substrate. Trichomes, layered hair-like epidermal growth, regulate leaf radiation and water absorption by directly absorbing moisture and nutrients and preventing evaporation. Orchids, such as native Earina, possess velamen roots layered in a loose sheath of perforated dead cells that quickly absorb rain and atmospheric water. Further adaptations may include succulence or specialised CAM photosynthesis.


Community dynamics are also influenced by vertical microclimates, such that epiphytic strata distribution is in response to light and moisture gradients. Sciophytic (shade-loving) species, often distinguished by a deficient cuticle, are sequestered to lower positions along the trunk, where still air maintains greater ambient moisture. Filmy ferns Tmesipteris tannensis, Loxogramme dictyopteris, and Blechnum nigrum typically inhabit these shadowed niches. Heliophilic (sun-loving) species are present through the upper canopy and in lower stations exposed to columns of light. They exhibit pronounced xeromorphic features such as a thickened cuticle and water storage tissues. Epiphytic heliophiles include orchids, Pyrrosia, and Astelia.


Aloft on yawning boughs, Astelia solandri cascades over a rising system of trunks and forking branches, an immense orb and center of life and arboreal biodiversity in this complex aerial kingdom.


An endemic perennial herb, kōwharawhara or perching lily is regarded as a nest epiphyte with ensiform (sword-shaped) leaves that guide rainwater toward its center. The foliage emerges from a densely tufted basal rosette, each narrow sheath arched and drooping (100-200cm long). A monocot, its linear fronds exhibit parallel venation with three less prominent striations recognisable on either side of the midrib. The singular spring green fronds are covered in fine felt scales giving the barest pearlescent effect on the undersides of leaves, though less obviously when mature. In sun, this Astelia may also blush a slightly reddish hue.


Referred to as tākahakaha while in flower, A. solandri displays sprightly and deeply fragranced panicles of tightly clustered flowers, similar in appearance to Cordyline,  through October-June. Dioecious, the female flowers range viridescent to pink, but male plants exhibit most alluring mauve flowers.


The inflorescence is 15-40cm long and emerges energetically from a 30-100cm peduncle (stalk). Small translucent green-ochre spherical berries, 4-5mm in diameter, develop between January and December. The shining and concealed globose seeds are less than 2mm long. Sweet and fleshy fruit is dispersed by frugivory, particularly among tūi, kererū, kākāriki, kākā and kōkako, endemic birds similarly attracted to the flowers' nectar.


Kōwharawhara inhabits humid coastal and lowland forests from sea level to montane altitudes in Te Ika a Māui (North Island), the west coast of Te Waipounamu (South Island), and Rakiura (Stewart Islands). These regions experience humid summers and mild, moist winters with only light frost. It can tolerate occasional, short-lived temperatures down to between -5 and -10°c, perhaps even lower if given shelter from cold drying winds. As epiphytic adaptations are associated with rupsetral growth, Astelia solandri can also be found growing terrestrially and as a lithophyte on shaded rock surfaces.


Though the substantial clusters seem unlikely and precariously perched, strong thick roots proceed from a short thickened stem and grasp the tree bark, anchoring the plant in the niches of extending limbs. Colonies often then arise and encircle the trunk. Where attached vertically to a trunk, the stem will angle upward and outward, leaning into the elements.


Its sculptural form provides essential arboreal habitat and resources for diverse specialised native birds, invertebrates, and arboreal lizards, including Moko kākāriki, Wellington green gecko (Naultinus punctatus); Mokopirirakau, arboreal gecko (Mokopirirakau granulatus); and the Pacific gecko (Dactylocnemis pacificus). Kārearea, the New Zealand falcon, does not build its own nest and may use Astelia in the canopies of emergent forest trees as high nesting platforms. The perching lily provides similar nesting habitats for ruru, morepork owls. The fountain at the base of its leaves further sustain birds, bats, reptiles, and insects during dry periods.


Its reservoir of water and detritus generates a micro-ecosystem that also develops close associations with shrubby epiphytes Griselinia lucida and Pittosporum cornifolium, which send feeder roots into the developing soils layered within the Astelia. Hanging clubmoss (Phlegmariurus varius), Hanging spleenwort (Asplenium flaccidum), and sickle spleenwort (A. polyodon) are often found draped from perching lily and similar nest epiphyte Astelia hastata, formerly Collospermum hastata (tank lily, widow maker).


Something like a keystone species, Astelia are indicative of established life in the canopy, inviting vertical complexity, resilience, and biodiversity to native forest ecosystems. It and other epiphytes are largely unseen, and under-observed, but integral to flora-fauna interactions, soil health, pollination, climate regulation, and water and nutrient cycling.


Although Astelia solandri is individually robust and long-lived, epiphytes are exceptionally vulnerable to climate change (temperature, water availability, etc), and deforestation. Small variations in humidity can disproportionately affect species distribution, with few able to acclimate to drier conditions.


Bush fragments, common remnant forest isolations in New Zealand's largely agricultural matrix, are too small to retain adequate moisture for epiphytic growth. And young, small trees inadequate for canopy communities. As the last plants to colonise a forest, epiphytes require 100 years to reestablish, 50 years beyond trees. More beneficial than planting new trees, conservation of old-growth forest is critical to protecting these sublime species and irreplaceable micro-ecosystems.


bottom of page